Your Gut Microbiome Is an Ecosystem — And That Changes Everything We Think We Know About ‘Good’ Bacteria
Oct 06, 2026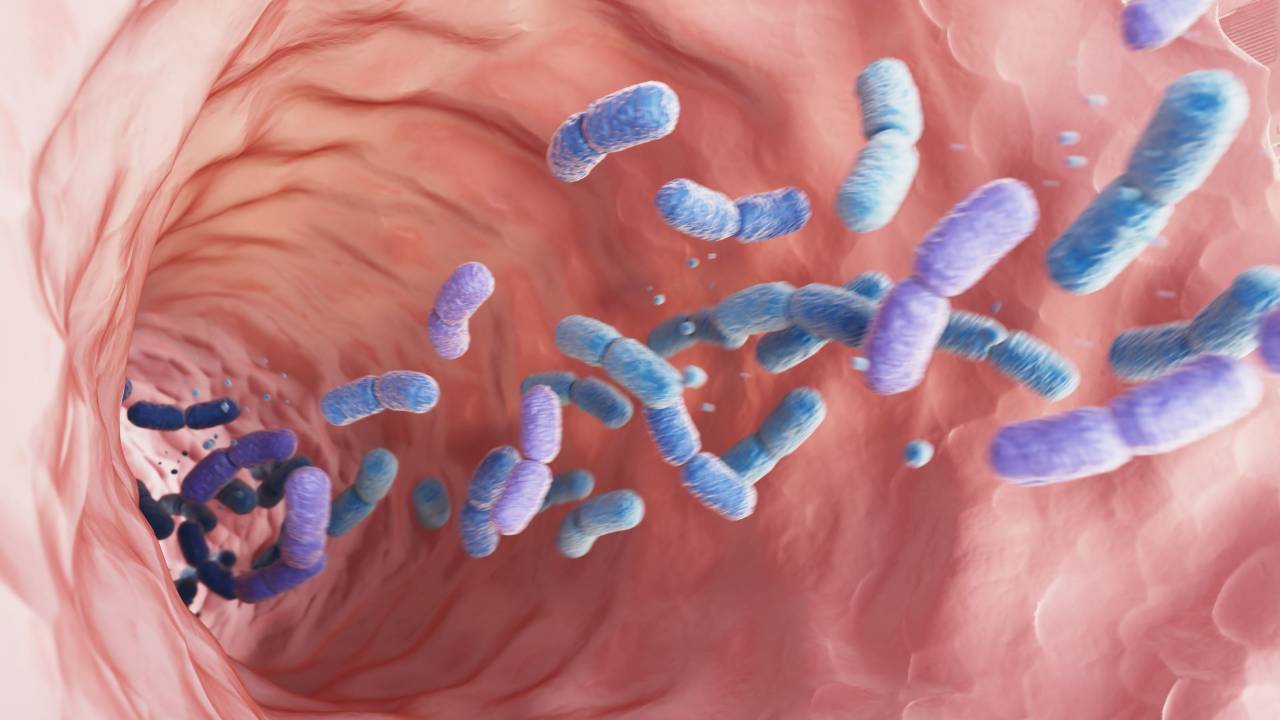
Gut-health advice has developed a rather neat little story over the last decade. Eat plenty of fibre, feed your good bacteria, avoid doing things that encourage the bad ones and, with a little luck and perhaps a suitably expensive probiotic, your microbiome will flourish.
It is an appealing idea because it makes an extraordinarily complicated biological system sound reassuringly manageable. Unfortunately, the organisms living inside the colon appear to have missed the memo.
The human gut microbiome is not a collection of individual bacterial species sitting independently beside one another waiting for us to deliver their favourite breakfast. It is a densely populated ecological community in which microorganisms compete for resources, share metabolites, modify one another's environment, communicate chemically, prey upon one another and alter their behaviour according to which neighbouring organisms happen to be present.
A fascinating study published in Nature Microbiology in October 2026 demonstrates this remarkably well. Researchers screened 94 dietary components to investigate why certain bacterial communities are dominated by Bacteroides-related organisms while others contain much larger populations of Segatella copri, formerly known as Prevotella copri.
Some complex plant carbohydrates dramatically increased S. copri. One particular polysaccharide, arabinan, increased its relative abundance from approximately 1.7% to almost 60% within a synthetic microbial community.
At first glance, this appears to fit the usual microbiome story perfectly. Give bacterium X its preferred fibre and bacterium X flourishes.
Then the researchers removed the rest of the microbial community.
Suddenly, the result changed.
When S. copri competed directly against Bacteroidaceae in isolation, the apparent advantage produced by arabinan disappeared. The carbohydrate alone was not enough. Other organisms within the community were helping determine who won the competition.
One group of bacteria turned out to be particularly important: Enterobacteriaceae, including strains of Escherichia coli. Adding them back into the experimental system restored the competitive advantage of S. copri across several different plant polysaccharides.
The lesson is much bigger than the fate of one bacterial species. It tells us that the physiological consequences of eating a fibre may depend partly upon which organisms are already living in the ecosystem that receives it.
That makes the usual instruction to “feed your good bacteria” look rather optimistic.
The microbiome is not an organ with a fixed membership list
When we talk about the gut microbiome, it is tempting to imagine a fairly standard collection of microorganisms that everybody possesses in slightly different proportions.
Reality is considerably messier.
Human gut microbial communities differ enormously between individuals. Geography, habitual diet, age, medication, early-life environment, infection, genetics, social environment and numerous other exposures can influence which organisms are present and what they are doing.
Even healthy people can possess strikingly different microbial communities.
Large-scale analyses have repeatedly shown broad differences between populations living traditional lifestyles and those living in industrialised societies. Bacterial groups including Prevotellaceae and Segatella tend to be considerably more abundant in many populations consuming traditional, fibre-rich diets, whereas members of the Bacteroidaceae are frequently more prominent in industrialised populations.
Diet undoubtedly contributes to these patterns, but diet alone does not explain them.
That is precisely what makes the new Nature Microbiology experiment interesting. The researchers were not simply asking which carbohydrate a particular bacterium could metabolise. They were asking why the same dietary substrate could produce different ecological outcomes depending upon the microbial community in which that organism was living.
That is a far more realistic representation of what happens inside the human colon.
Bacteria do not eat alone
Imagine placing twenty people into a kitchen containing a limited selection of ingredients. What each person ultimately eats would not depend only upon their own preferences. It would also depend upon what everybody else ate first, whether somebody transformed one ingredient into another, whether one person produced something another could use and whether a particularly aggressive individual nicked half the food before everybody else had reached the cupboard.
Microbial communities operate according to many of the same ecological principles, albeit without the inevitable argument over who finished the milk.
Different bacterial species possess different collections of enzymes that allow them to break down particular substrates. Some organisms can degrade complex polysaccharides that others cannot use directly. The metabolites produced during that initial degradation can then become food for another organism.
This process is known as cross-feeding.
Cross-feeding is one of the reasons the effect of a particular fibre cannot be predicted simply by asking which species is capable of breaking it down.
One organism may perform the initial degradation, another may consume an intermediate compound, and a third may convert the products into a metabolite such as butyrate. Hydrogen produced by fermentation may be consumed by completely different microorganisms, altering the thermodynamics of the original fermentation process and making it more favourable.
What looks from the outside like one bacterium “responding to fibre” may therefore involve an entire food web.
Fibre is not one substance either
The phrase “dietary fibre” creates another unfortunate impression of simplicity.
Fibre is not one nutrient behaving in one predictable manner. It describes a large and chemically diverse collection of carbohydrates and related compounds that resist digestion in the human small intestine to varying degrees.
Inulin behaves differently from resistant starch. Beta-glucans behave differently from arabinoxylans. Pectins, cellulose, fructo-oligosaccharides and the numerous structural polysaccharides found within intact plant foods differ in molecular structure, solubility, viscosity and fermentability.
Microorganisms differ in their capacity to use each of them.
In the new study, the researchers screened 79 complex dietary glycans alongside 15 vitamins. More than half of the tested glycans significantly increased S. copri within the synthetic community, particularly polysaccharides derived from plant, algal and bacterial sources. Yet the ecological outcome depended upon the other organisms present.
Arabinan provided a particularly striking example. In the full microbial community, its addition increased S. copri roughly 35-fold while substantially reducing the relative abundance of Bacteroidaceae. However, when researchers simplified the system and directly competed S. copri against selected Bacteroidaceae, the expected advantage disappeared.
The bacterium was perfectly capable of metabolising arabinan. So were some of its competitors.
The determining factor was not simply who could eat the carbohydrate.
It was how the community interacted while eating it.
Enterobacteriaceae changed the outcome
The researchers discovered that Enterobacteriaceae altered this competition in ways that favoured S. copri.
Adding E. coli to the simplified microbial community restored the ability of S. copri to dominate in the presence of arabinan. Similar effects were subsequently demonstrated with several different Enterobacteriaceae strains and several different plant-derived polysaccharides.
This was not simply an arabinan curiosity.
Amylose, amylopectin and several other complex carbohydrates also gave S. copri a competitive advantage in the presence of E. coli that did not occur in the same way when the supporting organism was absent.
The researchers used metatranscriptomics and metabolomics to investigate what was changing within these microbial communities. Their results suggested that Enterobacteriaceae were altering the metabolic environment in ways that influenced competition between the major bacterial groups.
This is microbial ecology rather than simple nutrition.
The carbohydrate provides the substrate, but the biological outcome emerges from interactions between organisms.
This creates an immediate problem for the idea of ‘good bacteria’
One of the most persistent habits in consumer gut-health discussion is dividing microorganisms into good and bad categories.
Some organisms certainly possess pathogenic potential, and particular microbial configurations can be associated with disease. Nobody needs to pretend that Salmonella is simply misunderstood.
But most members of the normal gut microbiota do not fit comfortably into a moral classification system.
Take E. coli.
The name frequently evokes food poisoning because pathogenic strains of E. coli can cause serious disease. Yet numerous E. coli strains live harmlessly within healthy intestines as normal members of the microbial community.
In the new experiment, Enterobacteriaceae helped create ecological conditions that favoured S. copri. Whether that is ultimately beneficial, harmful or largely neutral to the human host cannot be determined simply from the increase in one bacterial species.
Nor should S. copri automatically be considered a beneficial organism simply because it is associated with some traditional, plant-rich dietary patterns. Different strains may behave differently, and the organism has been associated with both potentially favourable metabolic characteristics and inflammatory conditions in different contexts.
The label attached to the bacterium tells us considerably less than we might like.
Function matters. Context matters. Increasingly, the community matters.
The same bacterium can behave differently in a different ecosystem
One of the reasons microbiome research is so difficult is that the behaviour of a microorganism is not fixed.
A bacterial genome provides metabolic potential, not a complete description of what the organism will actually do in every environment.
Gene expression changes according to available nutrients, pH, oxygen, neighbouring species, microbial metabolites and numerous other environmental signals.
A bacterium living inside one microbial community may therefore express a very different set of genes from the same species living within another.
Recent co-culture experiments have demonstrated just how dramatic these interactions can become. When researchers cultured human gut bacteria alongside different neighbouring species, large proportions of their proteome changed compared with when those organisms were grown alone. Proteins involved in nutrient transport and carbohydrate metabolism were particularly responsive to microbial neighbours.
This means that simply identifying a species in somebody's stool sample cannot tell us everything we would want to know about its behaviour.
Finding an organism tells us who appears to be present. It does not necessarily tell us what they are doing.
This is why function may ultimately matter more than a species list
Commercial microbiome testing has encouraged the idea that health can be inferred by identifying which organisms appear in somebody's stool and comparing their abundance with a supposedly optimal reference population.
There is scientific value in characterising microbial communities. In research, metagenomics and other sequencing technologies have transformed our understanding of the gastrointestinal ecosystem.
The leap occurs when those data are converted into highly specific dietary instructions for an individual.
The functional output of the microbiome depends upon far more than the relative abundance of named bacterial species. It depends upon strain-level variation, gene expression, substrate availability, microbial competition, cross-feeding and the biochemical environment created by the host.
Two people could possess different microbial communities yet produce similar metabolic functions because different organisms can perform overlapping tasks. This is known as functional redundancy.
Conversely, two people with apparently similar bacterial profiles could produce different metabolite patterns because those organisms are behaving differently.
This is why stool sequencing and microbial function should not be treated as interchangeable.
Knowing that somebody possesses a particular butyrate-producing bacterium does not automatically tell us how much butyrate is being produced.
The bacterium still needs an appropriate substrate. The surrounding microbial community can alter the pathway. The host may absorb the metabolite rapidly, meaning faecal concentrations do not accurately represent production. Other organisms may consume it.
The microbiome is not simply a census. It is an economy.
Cross-feeding explains why microbial metabolites cannot always be traced back to one food
Short-chain fatty acids provide a particularly useful example.
Acetate, propionate and butyrate are produced primarily through microbial fermentation of carbohydrates that escape digestion in the small intestine. These compounds have attracted enormous attention because they can interact with colonocytes, immune cells, enteroendocrine signalling and aspects of host metabolism.
The usual explanation is that fibre reaches the colon, beneficial bacteria ferment it and short-chain fatty acids appear.
That is broadly true, but the actual metabolic network can be considerably more complex.
Some primary fermenters break large polysaccharides into smaller molecules. Other organisms use those products and release lactate, acetate or succinate. Different bacteria can then convert those intermediates into butyrate or propionate.
An organism that ultimately produces butyrate may therefore depend upon another species to supply the substrate from which it makes it.
Removing one apparently minor member of the ecosystem can consequently change a metabolic output produced somewhere else.
This is another reason probiotic claims based upon one named organism need caution. Adding a bacterium to an established gut ecosystem does not guarantee that it will permanently colonise, obtain the substrates it requires or interact with the existing microbial community in the manner observed in a laboratory culture.
A living ecosystem has a habit of being rather less cooperative than a Petri dish.
Human fibre studies show enormous variation between individuals
The ecological model also helps explain something repeatedly observed in human dietary interventions: people can respond very differently to the same fibre.
A large randomised trial published in Nature Communications in 2025 enrolled 802 people with prediabetes and randomly assigned them to usual care or a dietary fibre intervention for six months.
When researchers examined the entire study population, the fibre intervention did not significantly improve the primary glycaemic outcome compared with the control condition.
That might appear to suggest that the fibre intervention simply failed.
The subgroup analyses told a more complicated story.
Participants could be divided into metabolic clusters that also possessed distinct microbiome profiles. Within two of those clusters, fibre supplementation was associated with improvements in glycaemic control and corresponding microbial changes, whereas participants in the other clusters showed little benefit.
Researchers then developed a microbiome-based score intended to predict who was more likely to respond and validated the model in additional fibre-intervention datasets.
This is extremely interesting, but it should not be oversold. The overall trial was negative for its primary comparison, while much of the personalised-response work was post hoc. The predictive model was developed largely within Chinese populations and requires much broader validation before anybody should be ordering a stool test to determine which breakfast cereal they need.
Nevertheless, the study supports the idea that baseline microbial ecology can influence the response to a nutritional intervention.
A smaller randomised trial examining resistant-starch-rich unripe banana flour and inulin similarly found that participants with different baseline microbial community structures responded differently. People with a Prevotella-rich microbiome showed considerably greater compositional and functional changes from the resistant-starch intervention than those with a Bacteroides-rich community.
The dietary exposure was the same. The starting ecosystem was not.
This does not mean we are ready for microbiome-personalised diets
The obvious temptation is to jump straight from this research into precision nutrition.
Send off a stool sample, identify your microbial community and receive a personalised menu telling you precisely which fibres your bacteria require.
For personalised microbiome nutrition to become clinically useful, predictive models need to work across different countries, ethnicities, diets and disease states. Measurements need to be reproducible over time. We need to know which microbial features actually cause differential responses rather than simply being associated with them.
We also need outcomes that matter.
Changing the relative abundance of a bacterial species is interesting. Improving HbA1c, cardiovascular risk, gastrointestinal symptoms or another meaningful health outcome is considerably more important.
The microbiome changes rapidly in response to diet, medication, illness and numerous environmental exposures. A single stool sample may therefore provide an incomplete snapshot of a dynamic ecosystem.
There is enormous promise here, but commercial enthusiasm is once again moving considerably faster than clinical validation.
If a company claims to know from one stool sample precisely which foods your body personally requires, I would keep one hand reasonably close to my wallet.
And then there are the viruses
If bacteria were not complicated enough, they are not the only inhabitants of the gut.
The gastrointestinal tract also contains enormous numbers of viruses, many of which are bacteriophages: viruses that infect bacteria.
The gut virome is increasingly emerging as another important layer of microbial ecology.
Bacteriophages can infect bacterial cells, replicate inside them and sometimes kill them. Other phages can integrate their genetic material into bacterial genomes and remain relatively dormant until environmental conditions change.
This means viruses can influence bacterial population size, gene expression and potentially the movement of genetic material between bacterial cells.
A new 2026 review focusing on colorectal-cancer biology has proposed that bacteriophages may act as ecological amplifiers, translating environmental disturbance into changes in bacterial behaviour, microbial metabolites, intestinal-barrier function and immune signalling.
Human studies have reported enrichment of particular lytic bacteriophages during colorectal adenoma development, raising the possibility that virome changes occur relatively early in some disease processes.
This remains emerging science. We certainly cannot conclude that particular phages cause colorectal cancer, nor can anyone sensibly prescribe a “virome diet” from these findings.
The broader lesson is much more useful.
Even when we think we are studying bacteria, there is another ecological layer influencing what those bacteria do.
Diet is therefore acting on a community, not delivering instructions to individual organisms
This changes how we should think about the relationship between nutrition and the microbiome.
When somebody eats onions, oats, lentils, beans, apples, whole grains or another fibre-rich food, that food is not sending a private biochemical message to one favoured bacterial species.
Different substrates enter a competitive microbial ecosystem.
Some organisms can degrade them directly. Others benefit from the breakdown products. Some compete for the same nutrients. Some consume metabolites produced by neighbours. Some alter pH or oxygen availability. Bacteriophages may affect bacterial abundance. The host simultaneously absorbs microbial metabolites and releases mucus, bile acids and other substances back into the environment.
The final biological output emerges from all of these interactions.
This is one reason nutritional interventions often produce heterogeneous microbiome results. A dietary change can be completely real while producing different microbial shifts in different people because their starting ecosystems are different.
Expecting one food to produce one universal microbiome signature may therefore be unrealistic.
What does this mean for prebiotics?
Prebiotics are substrates selectively utilised by host microorganisms that confer a health benefit.
The definition itself is important because simply demonstrating that a fibre increases a bacterial population does not establish that it is beneficial.
Inulin and fructo-oligosaccharides are probably the best-known prebiotic compounds, but research increasingly investigates resistant starches, galacto-oligosaccharides and numerous other carbohydrates.
Their effects can be very useful, but they are not necessarily uniform.
Someone beginning with a microbial community containing organisms capable of efficiently using a particular prebiotic may respond strongly. Another person may show relatively little compositional change. A third may generate different metabolites because cross-feeding networks differ.
Tolerance varies as well. Rapid fermentation can increase gas production, causing bloating and discomfort in some people even when the same substrate is well tolerated by others.
None of this means prebiotics are ineffective.
It means microbiome interventions operate inside an ecosystem, and ecosystems contain history.
Does this undermine ordinary advice to eat more fibre?
Not remotely.
There is a risk that microbiome complexity can be used to make nutrition unnecessarily complicated. If everybody responds differently to fibre, perhaps we should wait for a stool test before eating vegetables.
That would be an extraordinary conclusion.
Dietary fibre has well-established effects extending far beyond changes in named bacteria. Different fibres influence bowel function, stool bulk, gastrointestinal transit, glycaemic response, cholesterol metabolism and satiation. Fermentable fibres provide substrates for microbial metabolism, while less-fermentable forms have valuable physical effects within the gastrointestinal tract.
Large bodies of epidemiological and intervention research support diets containing plenty of fibre-rich foods.
The ecological complexity of the microbiome does not weaken that recommendation.
It explains why the microbial response to it is not identical in everybody.
For most people, consuming a diverse range of vegetables, fruits, legumes, whole grains, nuts and seeds remains a much more defensible strategy than attempting to micromanage individual bacterial species.
Variety also provides an array of different fibres and phytochemicals rather than repeatedly supplying one purified substrate. From an ecological perspective, that may be considerably more sensible than deciding that one supposedly beneficial organism needs to be fed the same isolated prebiotic every morning for the rest of time.
Microbial diversity is useful, but it is not a universal health score either
The concept of diversity has become another shorthand in gut-health marketing.
Greater microbial diversity is frequently described as synonymous with a healthier microbiome.
There is some justification for the interest. Reduced microbial diversity has been observed in several disease states, and diverse ecosystems can sometimes be more resilient to disturbance.
But diversity is not universally beneficial simply because the number is higher.
A community can contain many organisms and still include undesirable functional characteristics. Infants naturally have lower gut-microbial diversity than adults without being pathologically unhealthy. Some traditional populations can have extremely diverse microbial communities that look very different from those found in industrialised populations.
Even the meaning of “diversity” varies according to the measurement being used.
What we ultimately care about is whether the microbial ecosystem performs functions compatible with host health and remains appropriately resilient when challenged.
That requires considerably more information than counting species.
We may eventually treat the microbiome ecologically
One of the more exciting implications of this work is that future microbiome therapies may become less focused on adding one supposedly beneficial organism and more focused on engineering ecological conditions.
Instead of asking how to increase bacterium X, researchers may ask what combination of substrates and microbial interactions creates a stable community capable of producing a desired function.
That could involve combinations of prebiotics designed to alter resource availability, carefully selected microbial consortia rather than single-strain probiotics, bacteriophage therapies capable of targeting particular organisms or treatments that modify microbial metabolites rather than microbial membership.
Faecal microbiota transplantation already provides a dramatic example of ecosystem-level therapy. In recurrent Clostridioides difficile infection, transferring a complex microbial community can restore colonisation resistance far more effectively than trying to add one supposedly protective bacterium.
The success of that intervention illustrates an ecological principle. Sometimes the function we want belongs to the community, not to one microorganism.
Whether similar approaches can eventually be used safely and predictably for metabolic disease, inflammatory conditions or other disorders remains far less certain.
The future of gut health will probably involve function rather than bacterial celebrity
Consumer microbiome science has created its own collection of celebrity organisms.
Akkermansia muciniphila has become fashionable. Various Bifidobacterium and Lactobacillus strains occupy supplement shelves. Butyrate-producing organisms are routinely celebrated. Particular bacteria rise and fall in popularity according to whichever paper generated headlines that month.
These organisms can all be scientifically interesting.
The problem begins when interesting associations are converted into a universal hierarchy of good and bad microbes.
A microorganism exists inside an environment. Its behaviour depends upon available substrates, neighbouring species, host physiology and strain-level genetics. The metabolic products generated by the community can matter just as much as the organisms producing them.
Future microbiome medicine will therefore probably become less interested in asking whether everybody has enough of one fashionable species and more interested in understanding what the microbial community is capable of doing.
Metagenomics can tell us which microbial genes are present. Metatranscriptomics can reveal which genes are actively being expressed. Metabolomics can measure the small molecules being produced. Combining these approaches with information about diet and host physiology will provide a much richer picture than taxonomy alone.
That is considerably harder than producing a stool-test report containing green and red bars.
It is also considerably closer to the actual biology.
What should we do while the science catches up?
The reassuring part is that we do not need a detailed microbial map to look after the gastrointestinal ecosystem reasonably well.
A diverse diet containing plenty of minimally processed plant foods provides an equally diverse supply of fibres and phytochemicals capable of reaching the intestinal microbiota. Legumes, whole grains, vegetables, fruits, nuts and seeds offer different structural carbohydrates rather than one endlessly repeated substrate.
Fermented foods may contribute additional microorganisms and metabolites, although their effects vary substantially according to the product and individual.
Unnecessary antibiotic use should obviously be avoided, while clinically necessary antibiotics should equally obviously not be rejected because someone is frightened of disturbing their microbiome. Medicines exist to treat disease, not to preserve an idealised bacterial profile at all costs.
Regular physical activity, sleep and metabolic health may also interact with the gut environment, although none should be described as a simplistic method for “boosting good bacteria”.
For people with gastrointestinal disease, dietary interventions need considerably greater individualisation. Someone with inflammatory bowel disease, severe irritable bowel syndrome or another gastrointestinal condition should not be told simply to consume as much fermentable fibre as possible because fibre is supposedly good for the microbiome.
Context remains important here too.
Gut health is becoming more interesting as it becomes less simple
The early years of microbiome research necessarily focused on identifying which organisms were present and which were associated with health or disease. That work was transformative. For the first time, sequencing technologies allowed researchers to examine microbial communities that had previously been largely inaccessible.
The next stage is proving considerably more complicated.
We now know that organisms interact extensively. They exchange metabolites, compete for nutrients and modify one another's behaviour. Their genes are expressed differently according to the community around them. Viruses influence bacterial ecology. Diet alters substrate availability while the host simultaneously changes the environment through bile acids, mucus, immune signalling and gastrointestinal transit.
The recent Nature Microbiology study provides a particularly elegant demonstration of this complexity. A plant polysaccharide could dramatically favour S. copri within one microbial community but failed to produce the same competitive outcome when key supporting organisms were removed. The effect of the food depended upon the ecological context in which it arrived.
That finding should make us cautious about claims that one fibre, probiotic or food can reliably manufacture the same “healthy microbiome” in everybody.
It should not make us pessimistic.
Quite the opposite.
Understanding the microbiome as an ecosystem gives us a much better framework for eventually manipulating it intelligently. We may discover why one person responds beautifully to a particular fibre while another develops nothing more impressive than wind. We may learn how combinations of organisms cooperate to produce metabolites that affect human physiology. We may eventually develop treatments that reshape microbial communities with a level of precision that today's probiotics cannot approach.
For now, perhaps the most useful shift is conceptual. Rather than asking which individual bacteria we need to collect and which ones we need to eliminate, we should start thinking about the environment we are repeatedly creating for the entire community.
The gut microbiome does not appear to care very much about our desire for a tidy list of heroes and villains.
It behaves like an ecosystem.
Nutrition science will become considerably better at understanding it once we do the same.
References
Culp, E.J. and Goodman, A.L. (2023) ‘Cross-feeding in the gut microbiome: ecology and mechanisms’, Cell Host & Microbe, 31(4), pp. 485–499. doi:10.1016/j.chom.2023.03.016.
Delzenne, N.M., Bindels, L.B., Neyrinck, A.M. et al. (2025) ‘The gut microbiome and dietary fibres: implications in obesity, cardiometabolic diseases and cancer’, Nature Reviews Microbiology, 23, pp. 225–238. doi:10.1038/s41579-024-01108-z.
Li, Y., Liu, W., Tian, L. et al. (2026) ‘Bacteriophages as an ecological driver of bacterial carcinogenesis in colorectal cancer’, Journal of Translational Medicine. doi:10.1186/s12967-026-09043-8.
Song, D., Feng, G., Ma, Y. et al. (2025) ‘Gut microbiome predicts personalized responses to dietary fiber in prediabetes: a randomized, open-label trial’, Nature Communications, 16, 11506. doi:10.1038/s41467-025-66498-x.
Tawk, C., El Mouali, Y., Huang, K.D. et al. (2026) ‘Synergy between Enterobacteriaceae and diet mediates competition between dominant Bacteroidales in the human gut’, Nature Microbiology. doi:10.1038/s41564-026-02500-6.
‘Baseline intestinal microbiota composition influences response to a real-world dietary fiber intervention’ (2025) npj Biofilms and Microbiomes. doi:10.1038/s41522-025-00817-4.
Like nutrition? You'll probably love this.
New research. Emerging ideas. Fascinating physiology. And a proper look at what the science actually means — without the hype.
Join my newsletter for weekly nutrition research, recipes, articles and insights worth knowing about.
We hate SPAM. We will never sell your information, for any reason.